Professional Interests
Precise regulation of RNA polymerase II (Pol II) transcription is fundamental to gene expression, cell identity, differentiation, and adaptive responses, and its disruption contributes to diverse human diseases. My research seeks to define the molecular mechanisms that govern Pol II progression through two critical regulatory transitions: initiation-to-elongation and elongation-to-termination. A central focus is understanding how cyclin-dependent kinases (CDKs) and opposing phosphatases establish dynamic phosphorylation states that regulate Pol II pausing, elongation, and termination, and how these signaling circuits are integrated with chromatin and histone post-translational modifications. Using the genetically tractable fission yeast Schizosaccharomyces pombe, we investigate both promoter-proximal pausing and 3′ pausing at gene ends to uncover shared and distinct mechanisms controlling transcriptional transitions. Our studies combine classical and chemical genetics with genomic and proteomic approaches, including ChIP-seq, PRO-seq, NET-seq, RNA-seq, 3′ RNA-seq, and MNase-seq. By defining how kinase–phosphatase networks, transcription factors, and chromatin cues coordinately regulate Pol II dynamics, our goal is to uncover conserved mechanistic principles of eukaryotic transcriptional control and provide a foundation for understanding how their disruption contributes to disease.
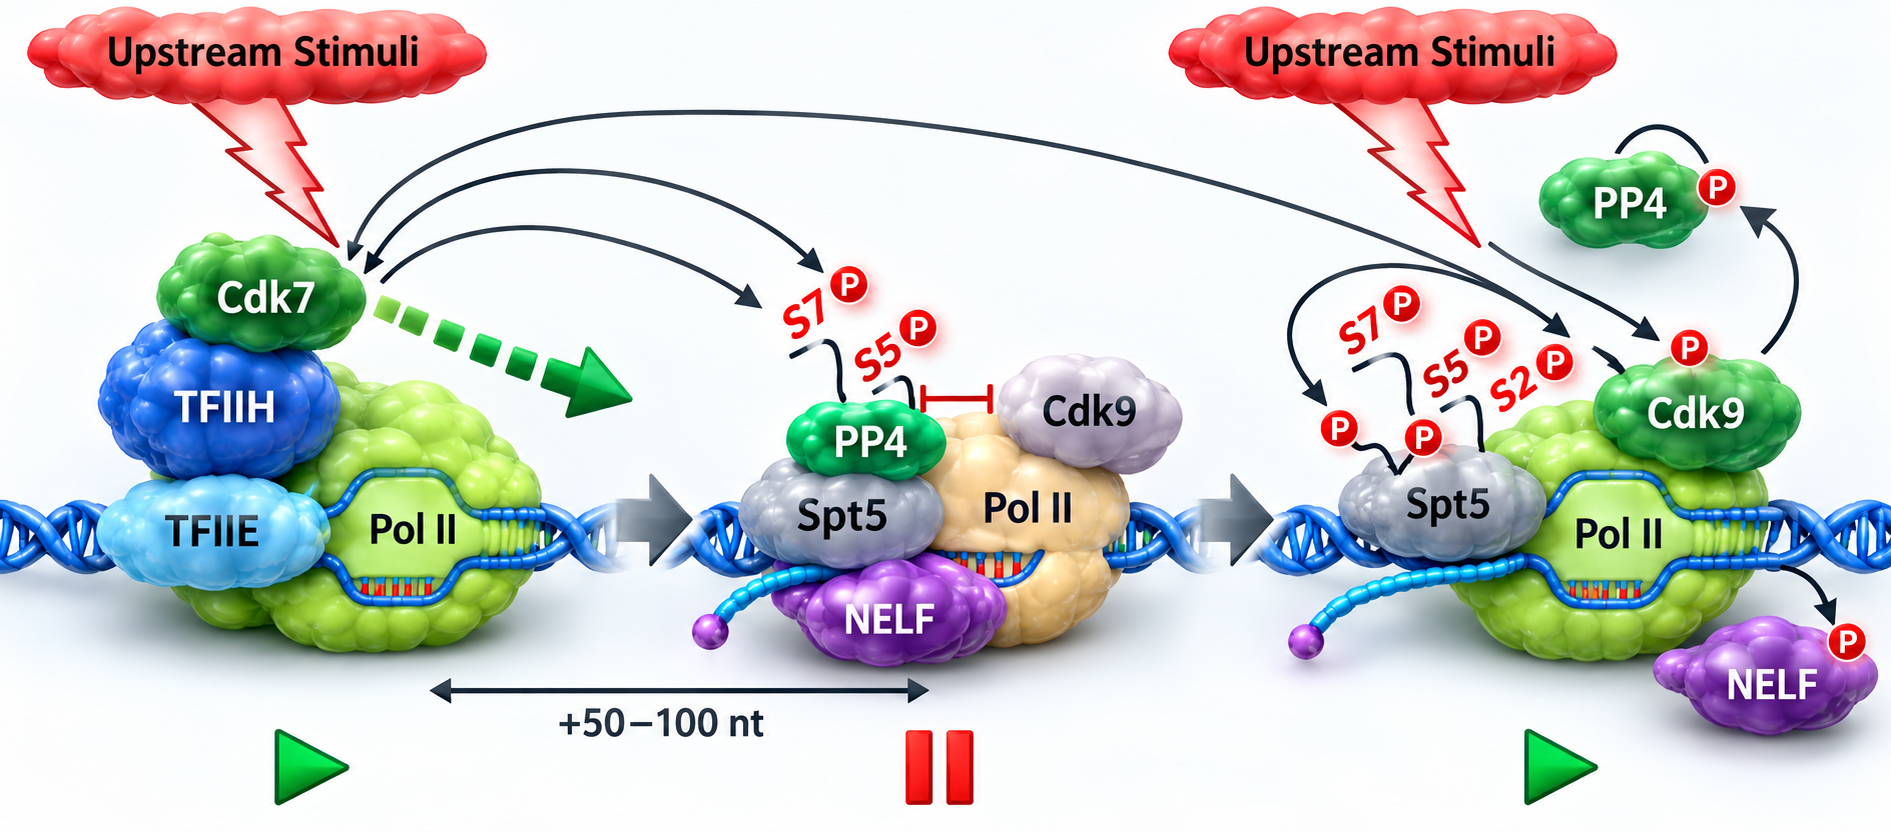
To obtain mechanistic insights into promoter-proximal pausing – Most of the genes in metazoan (and ~20% genes in fission yeast) are regulated by an early regulatory event, known as promoter-proximal pausing—Pol II is paused shortly after initiation around 20-80 nucleotides downstream of the transcription start site (TSS).Properly regulated release of stalled Pol II from the promoter-proximal pause site results in the synthesis of full-length transcripts. Mis-regulation of pausing or its release can result in abnormal gene expression. Given this early regulatory event’s decisive role in tuning Pol II transcription, dissecting the underlying molecular mechanisms is of utmost importance for understanding transcriptional homeostasis and its disruption in human diseases. Emerging studies suggest that the distinct kinase-phosphatase switch mechanisms control the phosphorylation of effector proteins, modulating the pause establishment, maintenance, and release. These critical kinase-phosphatase networks are mostly unknown and need to be identified and characterized precisely. We seek to investigate the regulation of promoter-proximal pausing in fission yeast and human cells to understand how the coordination between kinases and phosphatases ensures the pause establishment and synchronized release beneficial for healthy cells.
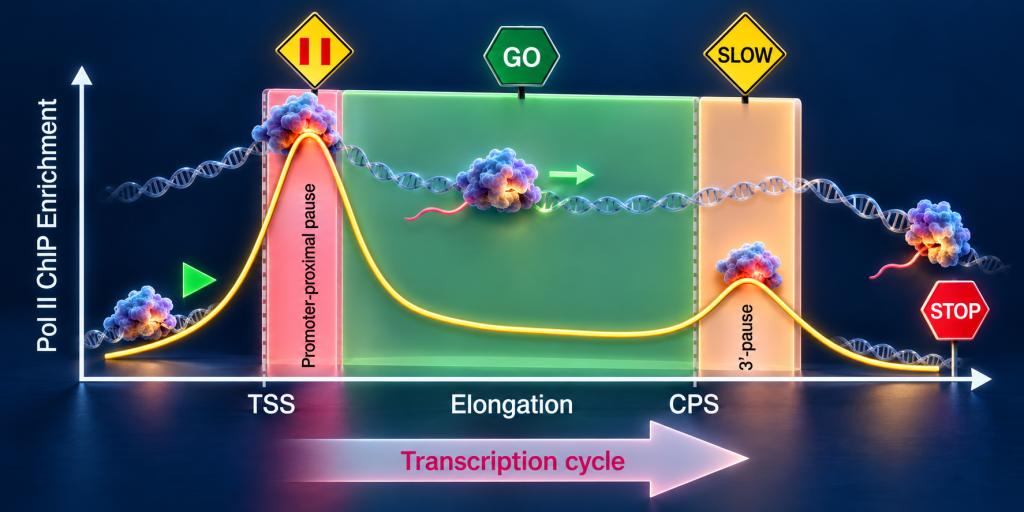
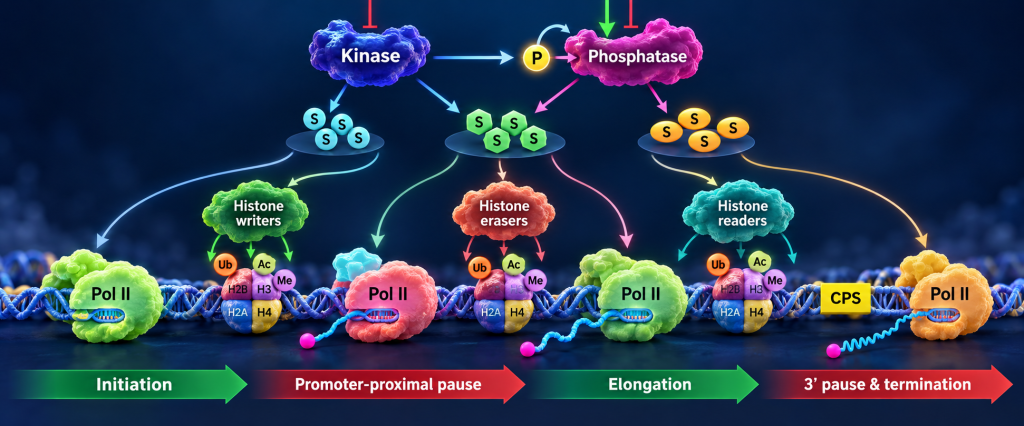
To investigate the coupling of transcription elongation and co-transcriptional processes – The variations in the rate of Pol II elongation have been implicated in controlling co-transcriptional processes such as 5′- and 3’-end processing, antisense transcription, alternative polyadenylation (APA), and splicing of pre-mRNA. However, much is still unknown, how the elongation rate is controlled and, consequently, the coupled process. The current hypothesis is that normal speeds of Pol II elongation favor the recruitment of factors necessary to execute a particular step, whereas slower Pol II promotes aberrant recruitment of factors, resulting in premature outcomes; conversely, faster rates impair the timely execution of exact steps. The primary objective here is to examine unidentified and uncharacterized connections among kinase-phosphatase antagonisms, rate of elongation, post-translational modifications (PTMs) of histones, pre-mRNA splicing, and transcription polarity.
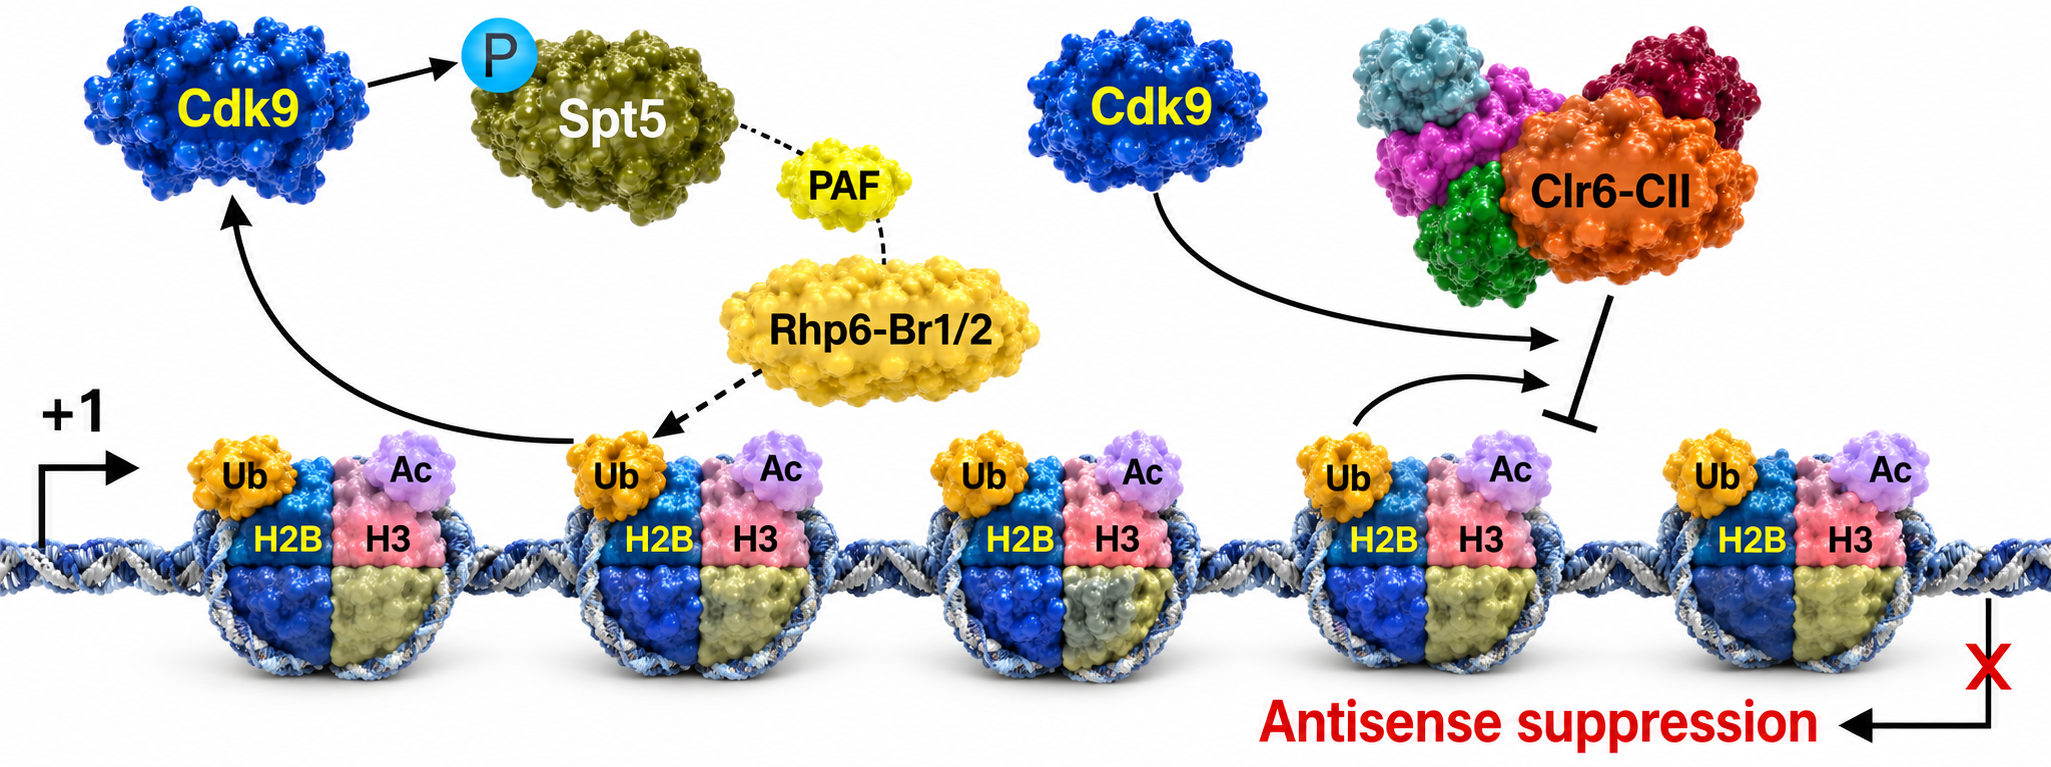
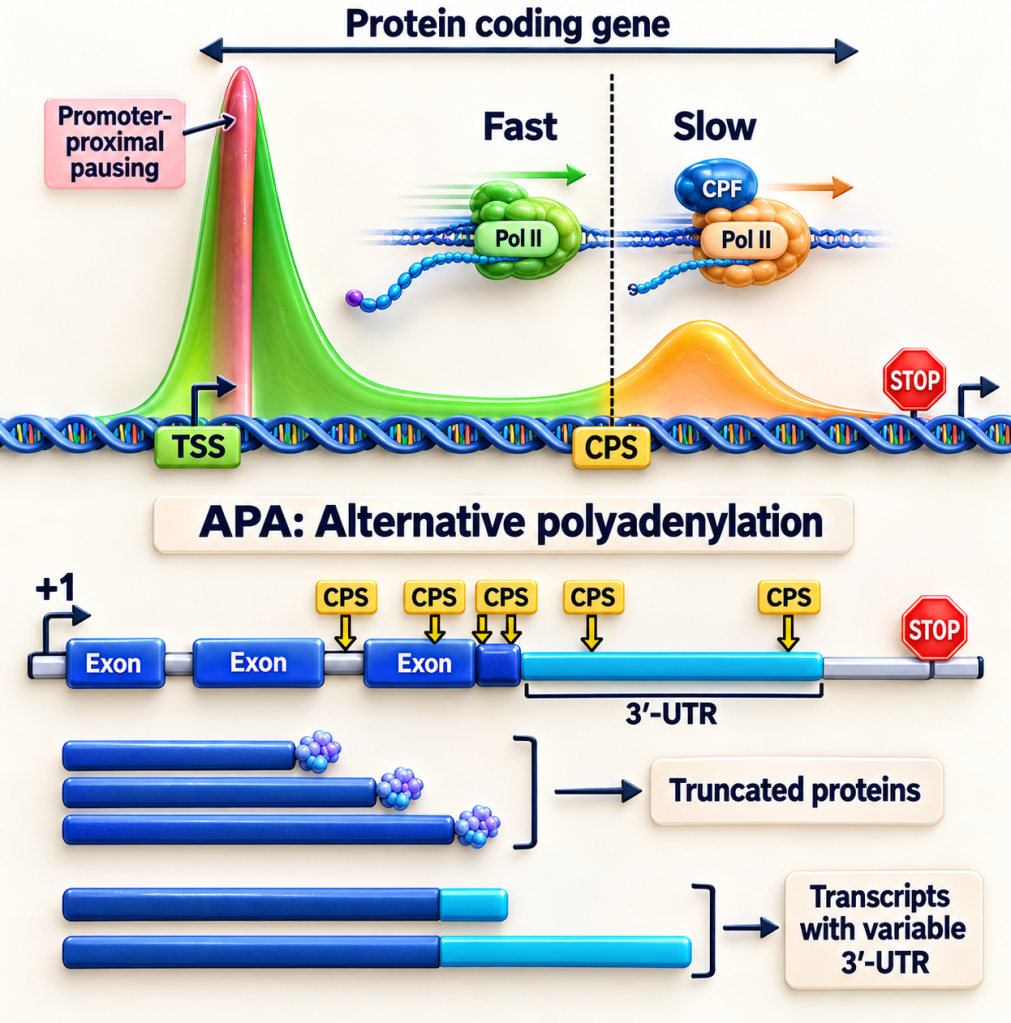
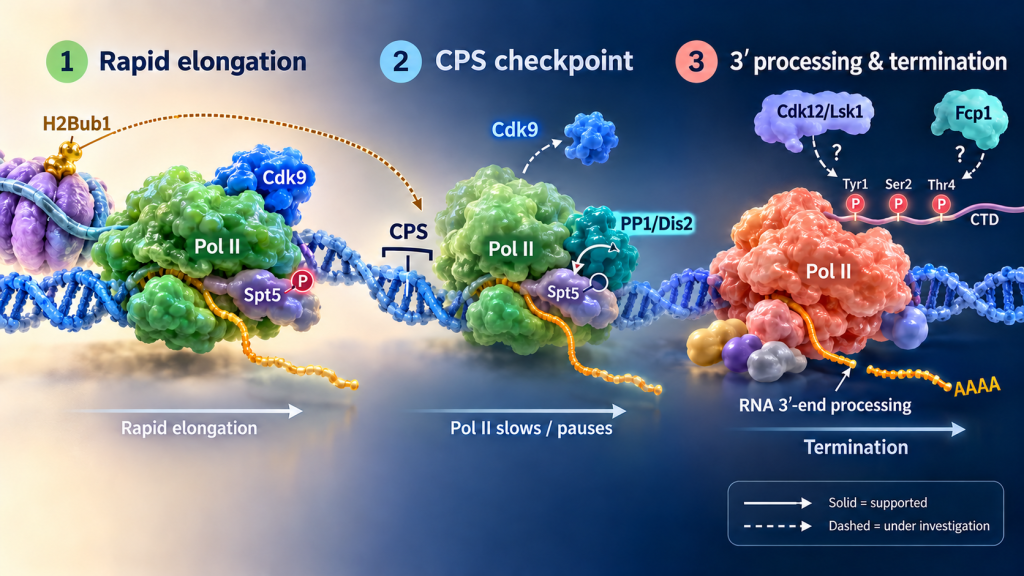
Decoding the Molecular Switches Governing the Elongation-to-Termination Transition — How does RNA polymerase II (Pol II) know when—and how—to stop transcription? Although transcription initiation and elongation are extensively studied, the molecular mechanisms that convert an actively elongating polymerase into a termination-competent complex remain poorly understood. Our research investigates the hypothesis that transcription termination is governed by an actively regulated checkpoint, coordinated through chromatin modifications and sequential kinase–phosphatase switches. As Pol II traverses the cleavage and polyadenylation signal (CPS), it slows, undergoes regulatory remodeling, and recruits RNA 3′-end processing and termination factors. We focus on two interconnected regulatory mechanisms. First, we investigate how histone H2B monoubiquitylation (H2Bub1) controls the Cdk9–PP1/Dis2 switch. Our recent findings demonstrate that H2Bub1 regulates Cdk9 disengagement and PP1 recruitment near gene ends, facilitating Spt5 dephosphorylation and productive termination. Second, we examine how opposing activities of Cdk12/Lsk1 and the phosphatase Fcp1 regulate Pol II C-terminal domain (CTD) phosphorylation at Tyr1, Ser2, and Thr4, potentially establishing a termination-competent phosphorylation state. Using Schizosaccharomyces pombe, we combine classical and chemical genetics, inducible protein degradation, targeted CTD mutations, and genome-wide genomic and proteomic approaches to dissect the causal relationships among chromatin signaling, kinase–phosphatase activity, Pol II dynamics, and RNA 3′-end formation. Our overarching goal is to establish a unified mechanistic framework for the elongation-to-termination transition, revealing how chromatin-encoded signals and dynamic phosphorylation coordinate transcriptional state changes. These studies may illuminate conserved principles of gene regulation and provide mechanistic insight into transcriptional readthrough and aberrant RNA 3′-end processing associated with human disease.